



Co-IP is the right protein-interaction method when an IP-grade antibody exists and the result needed is a wash-stable association around one bait. It is the wrong first method when the result needed is a binding constant, a contact residue, a live-cell proximity map, or a network built from one pellet. The real advantages of co-immunoprecipitation (Co-IP) are endogenous capture without a required tag, recovery of direct and bridged complex members, and a pellet that Western blot or mass spectrometry can read. The real disadvantages sit in the same chemistry: the assay is antibody-gated, lysis is not the living cell, the pellet is not a direct-binding proof, and Fc or resin binders travel with the bait. High specificity and “near-physiological” conditions are not properties of Co-IP. They are claims that have to be earned by the antibody, the buffer, and a matched control.
Specificity can still fail after a good antibody if the wash is unmatched. Indirect partners are expected in a true complex. They are not a detection gap.
If the question is already a nominated pair or an open partner list, researchers can review the MtoZ Biolabs Co-Immunoprecipitation Protein Interaction Analysis Service for project-specific feasibility and analysis planning.
Each advantage below applies only when the condition named with it is true. These are not automatic properties of Co-IP.
1. Endogenous bait, if an IP-grade antibody exists
Co-IP can capture an untagged protein from a cell or tissue lysate. That avoids an overexpression tag when the antibody is validated for immunoprecipitation. No antibody, or an antibody that only works on a denatured blot, removes this advantage. A Flag, HA, Myc, or GFP handle is then a different assay, not a more physiological Co-IP.
2. Complex-level recovery, including bridged subunits
While the antibody occupies the bait, proteins that remain attached through lysis and wash are collected. Direct contacts and intermediate-bridged subunits can both appear. That is an advantage for inspecting a complex and a disadvantage when the question is a binary interface. Co-IP recovers an indirect neighbor that stayed on the bait. It does not prove that the neighbor touches the bait directly.
3. Two readouts from one pellet
Western blotting tests a nominated prey. Mass spectrometry opens a peptide-identified list. The same capture principle supports both. MS does not identify every physiological component, and a Western band does not open the rest of the pellet. Versatility is the choice of readout, not a guarantee of a network. The capture steps are explained in Principle of Co-Immunoprecipitation in Protein Interaction Analysis.
4. Broad sample class, not a universal matrix
Lysates from cultured cells and from tissues can be used. Purified complexes can be re-bound only if the antibody still sees the epitope. “Applicable across samples” does not mean one buffer fits a membrane protein, a nuclear complex, and a secreted factor.
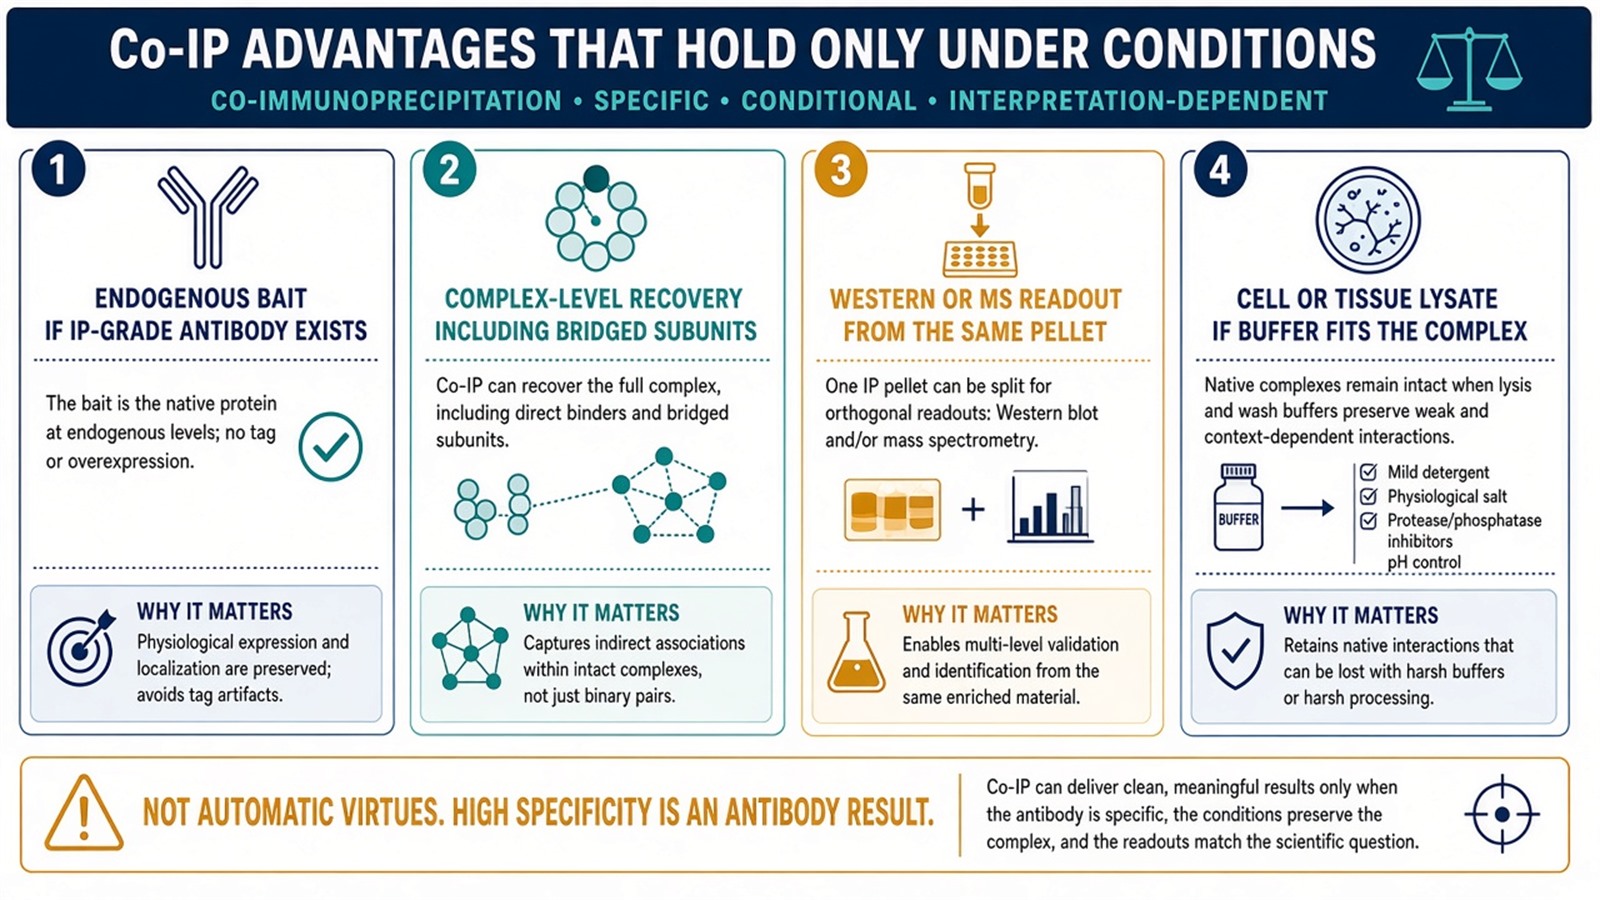
Figure 1. Endogenous capture, complex-level recovery, and a Western or MS readout are advantages only under those conditions. They are not automatic properties of Co-IP.
Structural Limits of Co-IP
These limits remain after a careful protocol. They are not beginner errors.
1. Antibody dependency
Capture stands or falls with epitope access, species, isotype, and affinity. A low-specificity antibody raises background. A low-affinity antibody misses the bait. Tagging removes the endogenous advantage and introduces tag binders. This is the central operational cost of Co-IP, not a side note.
2. Lysis is not the cell
Opening the cell dilutes local concentration and replaces cytoplasm with detergent and salt. A mild buffer is less denaturing than SDS. It is not a physiological environment. Interactions that needed membranes, organelles, or crowding can disappear. Interactions that form only after lysis can appear. “Physiological relevance” as an inherent advantage overstates the tube.
3. The pellet is not a direct contact
Co-recovery reports association that survived the wash. Bridged subunits, antibody-scaffold binders, and resin binders can occupy the same eluate. Reciprocal Co-IP strengthens a nominated pair. It still does not report a residue or a Kd. Why Co-IP-MS does not map binding sites is explained in Can Co-IP Followed by Mass Spectrometry Determine the Binding Sites Between Two Proteins?.
4. Background is part of the capture
A crowded lysate, Protein A/G surfaces, and Fc scaffolds collect proteins that never touched the bait. Washing reduces that class. It does not create a noise-free pellet. Signal classes that remain after washing, and how to change one variable at a time, are covered in How to Reduce High Background Signals in Co-IP Assays?
5. Occupancy limits low-abundance partners
A scarce prey is missed when few bait molecules are occupied, even if the antibody is adequate. Sensitivity is not a built-in Co-IP strength. Occupancy limits for low-expression proteins are covered in Co-IP for Low-Expression Protein Interactions.
6. Transient contacts are wash-sensitive
Weak or short-lived pairs fall off when salt or detergent is raised to clear background. Keeping them requires a milder wash and a stronger control comparison. Crosslinking before lysis is a different method, not a Co-IP upgrade. When the question is residue proximity, compare the workflows in Co-IP-MS vs XL-MS: Which Protein Interaction Workflow Should You Choose?.
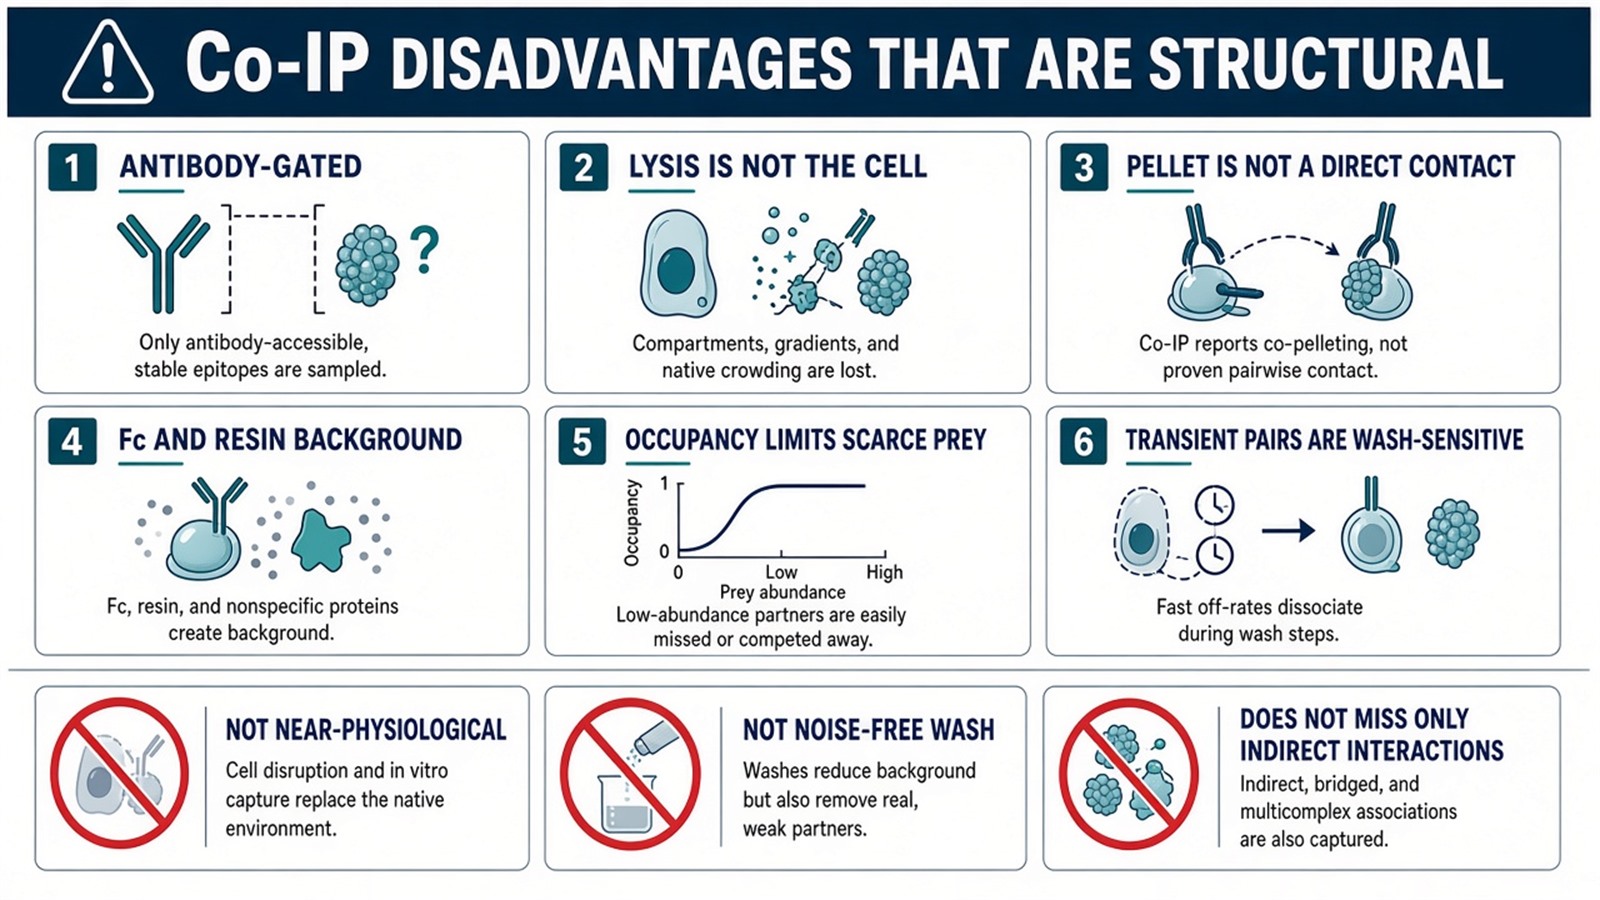
Figure 2. Antibody quality, non-physiological lysis, indirect and background proteins in one pellet, and low occupancy are structural limits. They are not fixed by calling the method native.
When Co-IP Is the Wrong First Method
Choose another assay when the decision already names a different physical event.
A binding constant needs SPR, BLI, ITC, or MST on defined components. A contact residue needs crosslinking MS, mutagenesis with an orthogonal readout, or a structure. A live-cell neighborhood that does not survive lysis needs BioID, TurboID, APEX, or in-cell XL-MS. A binary screen in a heterologous system is yeast two-hybrid territory, with its own false-positive class.
Co-IP remains useful after those methods, as an orthogonal co-recovery check. It should not be asked to replace them.
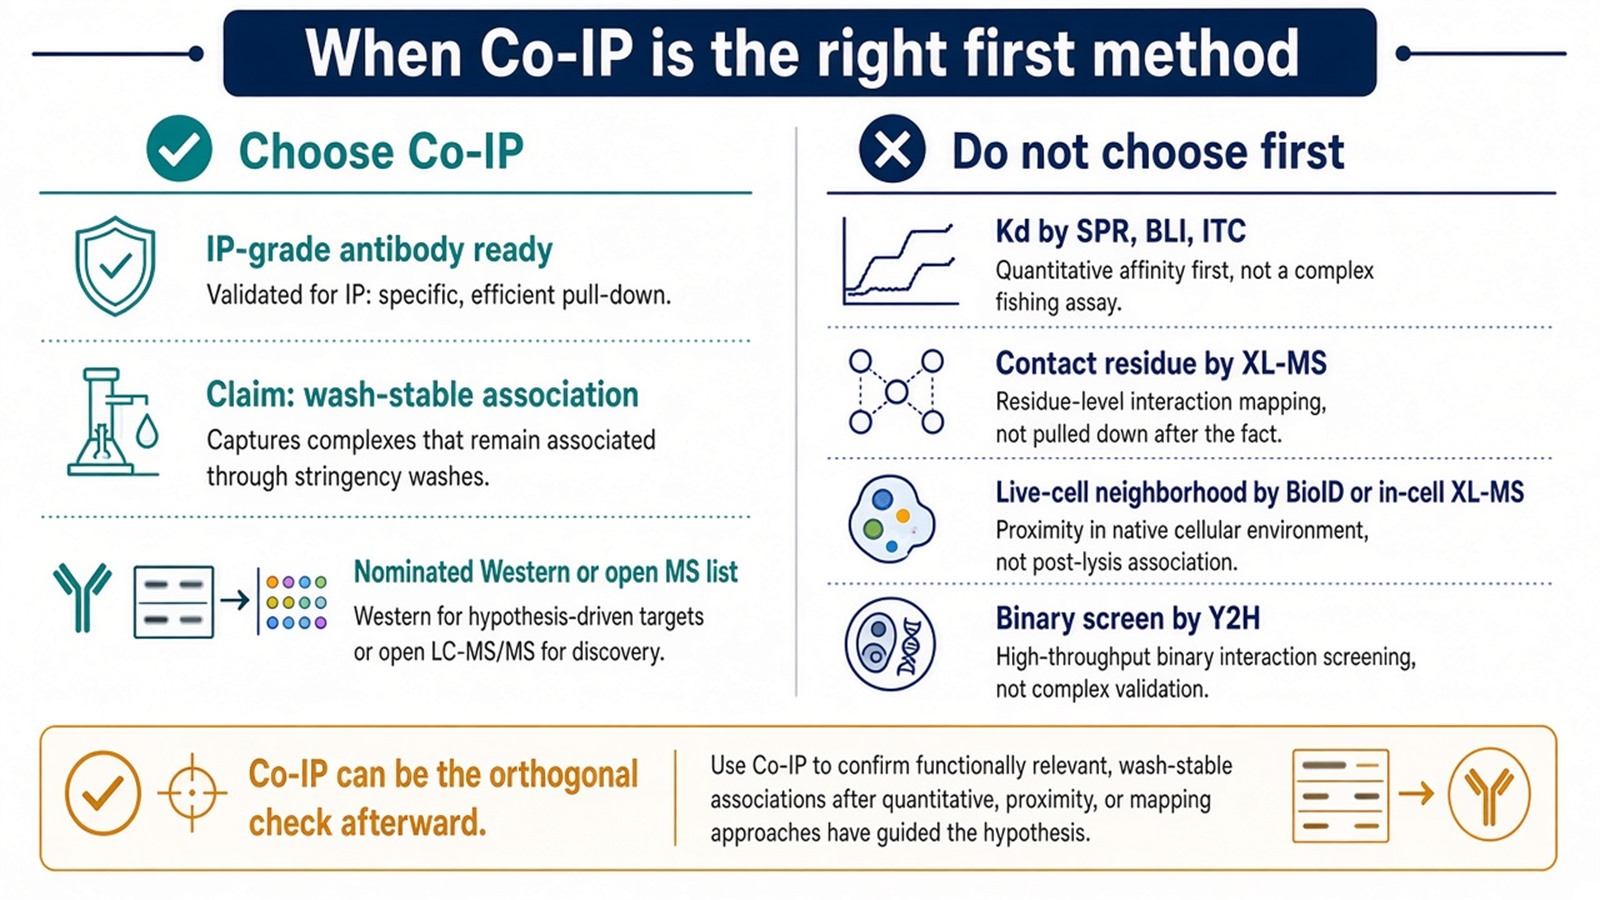
Figure 3. Use Co-IP when an IP-grade antibody exists and the readout is co-recovery. Use a biophysical, crosslinking, or proximity method when the question requires more than a pellet.
Common Mis-statements
“High specificity” is an antibody result, not a Co-IP advantage.
“Near-physiological” describes a milder buffer than SDS. It does not describe the living cell.
“Co-IP misses indirect interactions” is backwards. Co-IP recovers complexes. It does not prove a direct pair.
“MS identifies all components of the complex” over-reads an eluate list.
“Optimizing the wash removes background” over-reads a trade-off. Harsh washes also strip true partners.
Controls and Reporting Limits for Co-IP
The same pellet can contain bait-dependent partners and antibody- or bead-dependent background. A matched IgG or isotype control, or a beads-only or empty-tag arm when that arm fits the bait, shows which bands are not bait-dependent. Diagnostic cutoffs and clinical claims sit outside ordinary research reporting unless a separately validated assay framework is in place.
How to Plan a Co-IP or Co-IP-MS Project
A usable plan names the question first, then asks whether Co-IP’s advantages apply and whether its structural limits are acceptable. MtoZ Biolabs discusses endogenous or tagged Co-IP, and Co-IP-MS, when the question is wash-stable association around a defined bait. Interpretability still follows the antibody, the wash, and the control, not the instrument name.
Once those limits are acceptable, the project can be a nominated pair or an open partner list. Researchers who need LC-MS/MS on a Co-IP pellet after that decision can review the MtoZ Biolabs Co-IP-MS Protein Interaction Analysis Service for project-specific sample evaluation, feasibility assessment, and workflow planning.
Frequently Asked Questions
1. What is the main advantage of Co-IP?
Endogenous, complex-level co-recovery when an IP-grade antibody exists, with a pellet that Western or MS can read. Without that antibody, the endogenous advantage is gone. Without a matched control, the pellet cannot be assigned to the bait.
2. What is the main disadvantage of Co-IP?
The assay is antibody-gated, the tube is not the cell, and the pellet mixes true complex members with Fc and resin binders. Those are structural, not beginner, limits.
3. Does Co-IP detect only direct interactions?
No. Direct and bridged proteins can both co-precipitate. Direct contact needs an orthogonal assay.
4. Is Co-IP sensitive enough for low-abundance proteins?
Only when bait occupancy and detection depth are sufficient. Low expression is a common miss, not a hidden strength of the method.
5. Should Co-IP be the first PPI method?
Use it first when an IP-grade antibody is ready and the question is wash-stable association around one bait. Do not use it first for a Kd, a contact residue, or a live-cell map.
Reference
- Phizicky E.M., Fields S. (1995). Protein-protein interactions: methods for detection and analysis. Microbiol. Rev., 59, 94-123. https://doi.org/10.1128/mr.59.1.94-123.1995
- Berggård T., Linse S., James P. (2007). Methods for the detection and analysis of protein-protein interactions. Proteomics, 7, 2833-2842. https://doi.org/10.1002/pmic.200700131
- Gingras A.C., Gstaiger M., Raught B., Aebersold R. (2007). Analysis of protein complexes using mass spectrometry. Nat. Rev. Mol. Cell Biol., 8, 645-654. https://doi.org/10.1038/nrm2208
- ten Have S., Boulon S., Ahmad Y., Lamond A.I. (2011). Mass spectrometry-based immuno-precipitation proteomics: the choice of method matters. Proteomics, 11, 1153-1159. https://doi.org/10.1002/pmic.201000548
- Lin J.S., Lai E.M. (2017). Protein-protein interactions: co-immunoprecipitation. Methods Mol. Biol., 1615, 211-219. https://doi.org/10.1007/978-1-4939-7033-9_17
