



MiniTurbo proximity labeling uses a truncated biotin ligase, not the full TurboID enzyme. The two constructs share biotin-AMP chemistry and streptavidin recovery for liquid chromatography–tandem mass spectrometry (LC-MS/MS). They do not share size, residual labeling before biotin is added, or stability in a long 37 °C culture. MiniTurbo is smaller, about 28 kDa, because it lacks the N-terminal domain retained in TurboID, about 35 kDa. It often biotinylates less before the pulse. It is also less active during the pulse and can lose activity if the fusion sits in culture for many hours. The table is a neighborhood or a compartment proteome. It is not an interaction network, a topology map, or a nucleic-acid interactome. Proteins that sit close to the ligase can be labeled whether or not they bind the cargo.
Labeling happens in the living cell. Enrichment does not. After the pulse the cell is still lysed and streptavidin beads recover biotinylated proteins. Cloning the TurboID coding sequence into the same plasmid does not produce MiniTurbo. A localization-matched MiniTurbo without cargo is the control. Empty vector without enzyme does not estimate ligase background.
Researchers who already have a MiniTurbo fusion and need a streptavidin table can also review the MtoZ Biolabs miniTurbo Proximity Labeling Analysis Service for project-specific feasibility and analysis planning.
What MiniTurbo Is, and What It Shares with TurboID
MiniTurbo was engineered from the TurboID lineage by removing the N-terminal domain of Escherichia coli BirA and retaining a set of activity mutations. Inside the cell the fusion uses ATP to convert biotin into biotin-AMP. That mixed anhydride covalently tags nearby lysines. Streptavidin-coated beads then enrich those proteins. The original biotin-AMP description remains the chemistry. The original claim that MiniTurbo is TurboID does not.
BioID still uses the BirA* mutant over many hours. TurboID still uses the full faster ligase over about ten minutes and often a larger ligase-only proteome. MiniTurbo can also complete a pulse in about ten minutes when the enzyme remains active. Speed versus BioID is not its distinguishing property. A quieter baseline before biotin is added, and a smaller fusion, are. For the BioID-versus-TurboID comparison that does not decide MiniTurbo, BioID&TurboID provides a complementary ligase page. For the family that also includes APEX2, Proximity Labeling Mass Spectrometry provides a complementary ligase-versus-peroxidase overview.
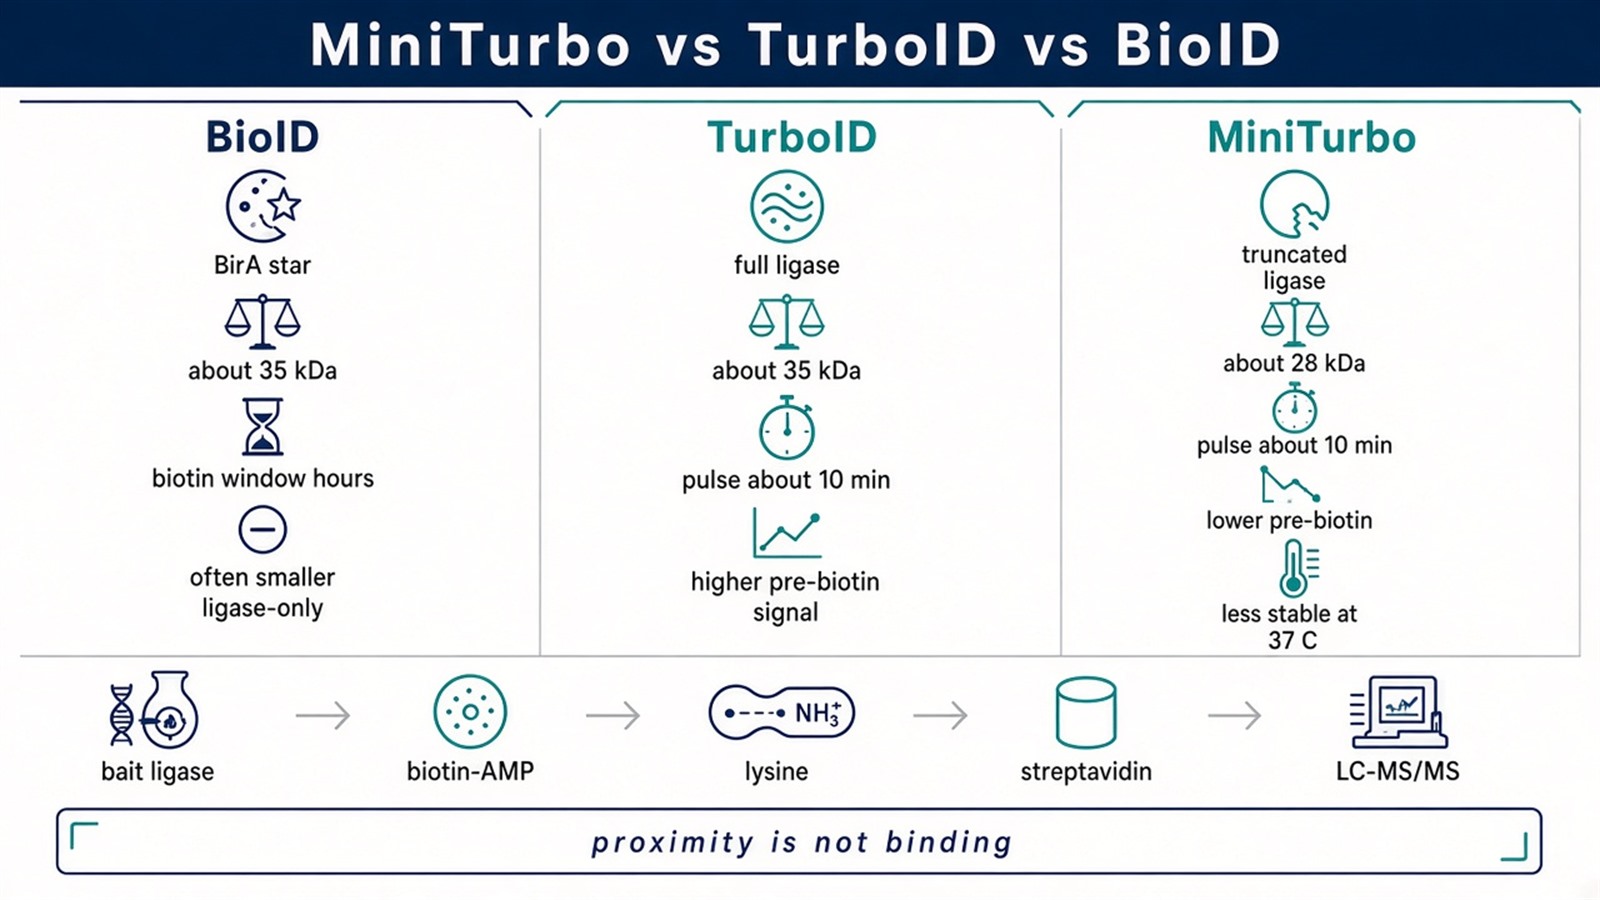
Figure 1. Shared path: bait-ligase, biotin-AMP, lysine, streptavidin, LC-MS/MS. MiniTurbo is smaller than TurboID and often quieter before biotin. It is not the TurboID coding sequence.
Clone MiniTurbo when the next sentence needs a smaller fusion or a quieter pre-biotin baseline. Clone TurboID when the next sentence needs more activity in a long culture.
When MiniTurbo Is the Better First Choice
These advantages hold only with the condition in the same sentence.
A ten-minute biotin pulse is available with MiniTurbo if the fusion is still active. That is not a guaranteed improvement in experimental efficiency over BioID, and it is not faster than TurboID. TurboID is usually the more active enzyme on the same bait.
Pre-biotin background can be lower with MiniTurbo if residual labeling from endogenous biotin is the problem being solved. That is temporal control of when biotinylation starts. It is not high specificity, and it is not precise capture of protein interactions at a defined time point. Specificity is still the ligase-only comparison after the pulse.
Fusion size can matter if the bait is cramped at a membrane, a contact site, or a small nuclear protein. MiniTurbo is useful there as a smaller handle. Size does not determine membrane-protein topology or name surface-exposed subunits. Lysine biotinylation near a localized ligase is not a topology assay.
Hydrogen peroxide is not required. Unlike APEX2, MiniTurbo does not use an H₂O₂ pulse. That avoids an oxidant bolus. It does not place the experiment in a physiological state, and it does not convert the table into native protein-protein interactions. For a one-minute tyrosine pulse that does use H₂O₂, APEX Proximity Labeling provides a complementary peroxidase option.
Weak, transient, or hydrophobic neighbors can receive biotin if they sit near the ligase during the pulse. Co-immunoprecipitation is not limited to high-affinity pairs, and MiniTurbo does not discover previously undetectable interactions by default. A labeled neighbor is a proximity candidate. For the low-copy use of the more active ligase, How Can TurboID-Based Proximity Labeling Enable the Study of Low-Abundance Protein Interactions? provides a complementary TurboID page.
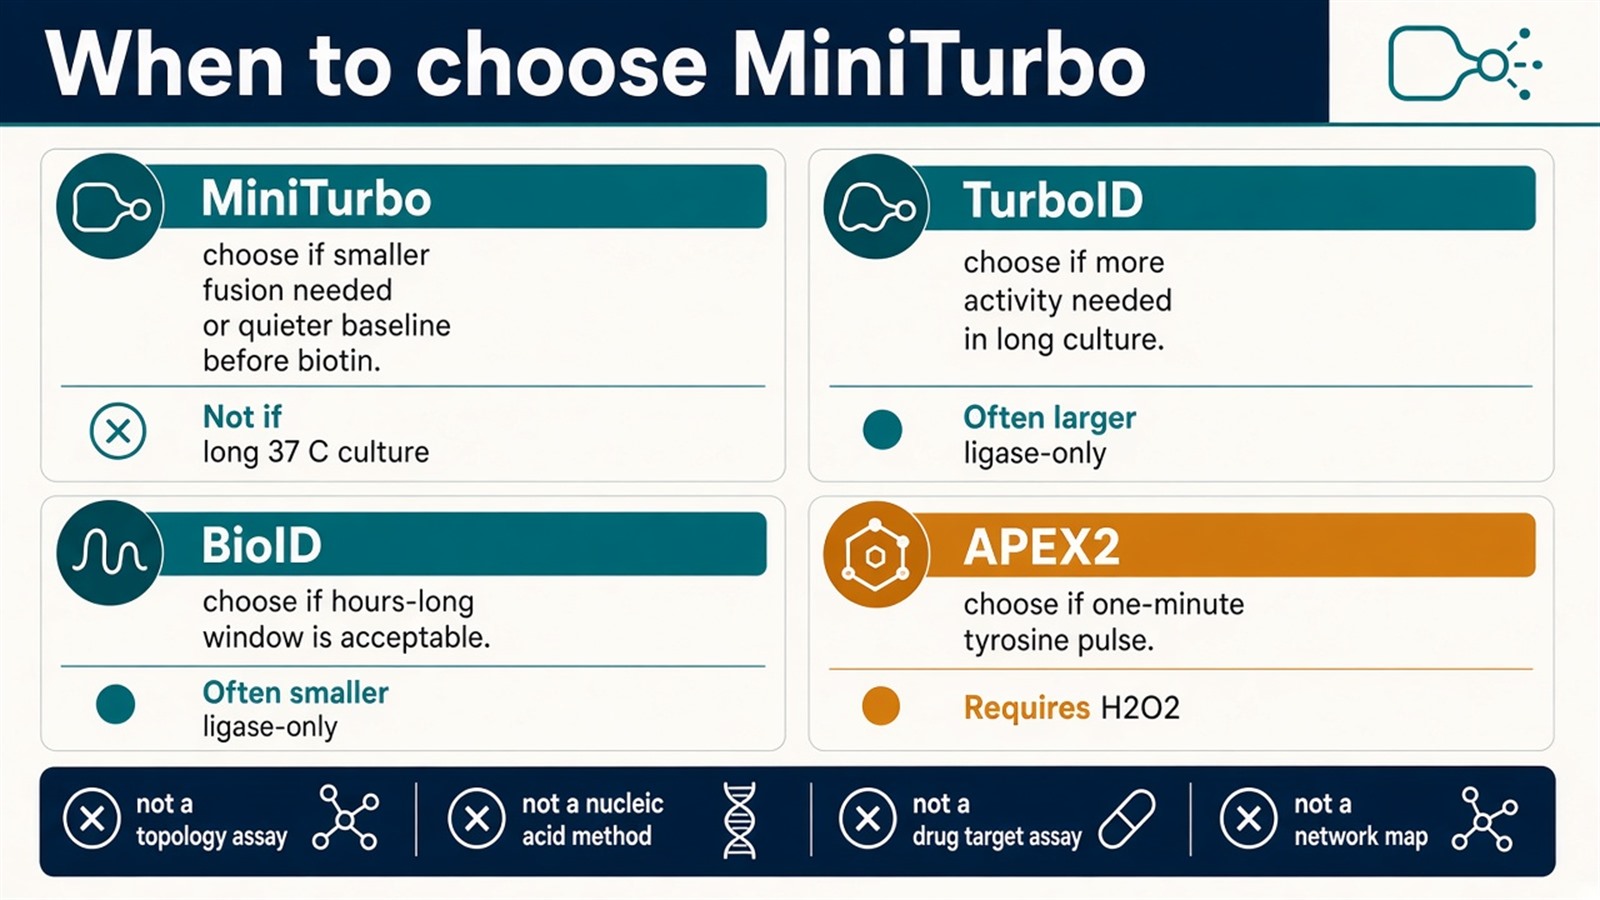
Figure 2. MiniTurbo: smaller handle, often lower pre-biotin signal, less stable at 37 °C. TurboID: more activity in long culture. BioID: hours. APEX2: tyrosine plus H₂O₂.
Workflow of MiniTurbo Proximity Labeling
The original four bench steps remain. The enzyme name and the control do not.
1. Genetic engineering and plasmid construction
The MiniTurbo coding sequence is fused to the bait or a localization sequence. The plasmid must express MiniTurbo, not TurboID. Folding and ligase activity are checked on the fusion that will be used. A localization-matched MiniTurbo without cargo is built at the same time. Adding that arm after a single bait digest cannot reconstruct background.
2. Cell transfection and expression check
The plasmid is introduced by lipid transfection, electroporation, or a comparable route. A stable line is useful only if MiniTurbo remains active after prolonged culture at 37 °C. MiniTurbo is less stable than TurboID in that setting. Localization is checked on the same cells before biotin is added. Consistent expression is not the same as a usable neighborhood.
3. Biotinylation and streptavidin capture
Biotin is added, typically for minutes when the enzyme is active. The pulse is a time window, not a physiological-condition guarantee. After lysis, streptavidin beads capture biotinylated proteins. Endogenous biotinylated carboxylases appear in both arms. They are expected rows.
4. Mass spectrometry analysis
The streptavidin eluate is analyzed by LC-MS/MS. Gel separation before the search is optional, not required. The search names proteins in the digest. It does not quantify a protein interaction network. Each row is first asked whether MiniTurbo or bait was recovered and whether the candidate is enriched against ligase-only.
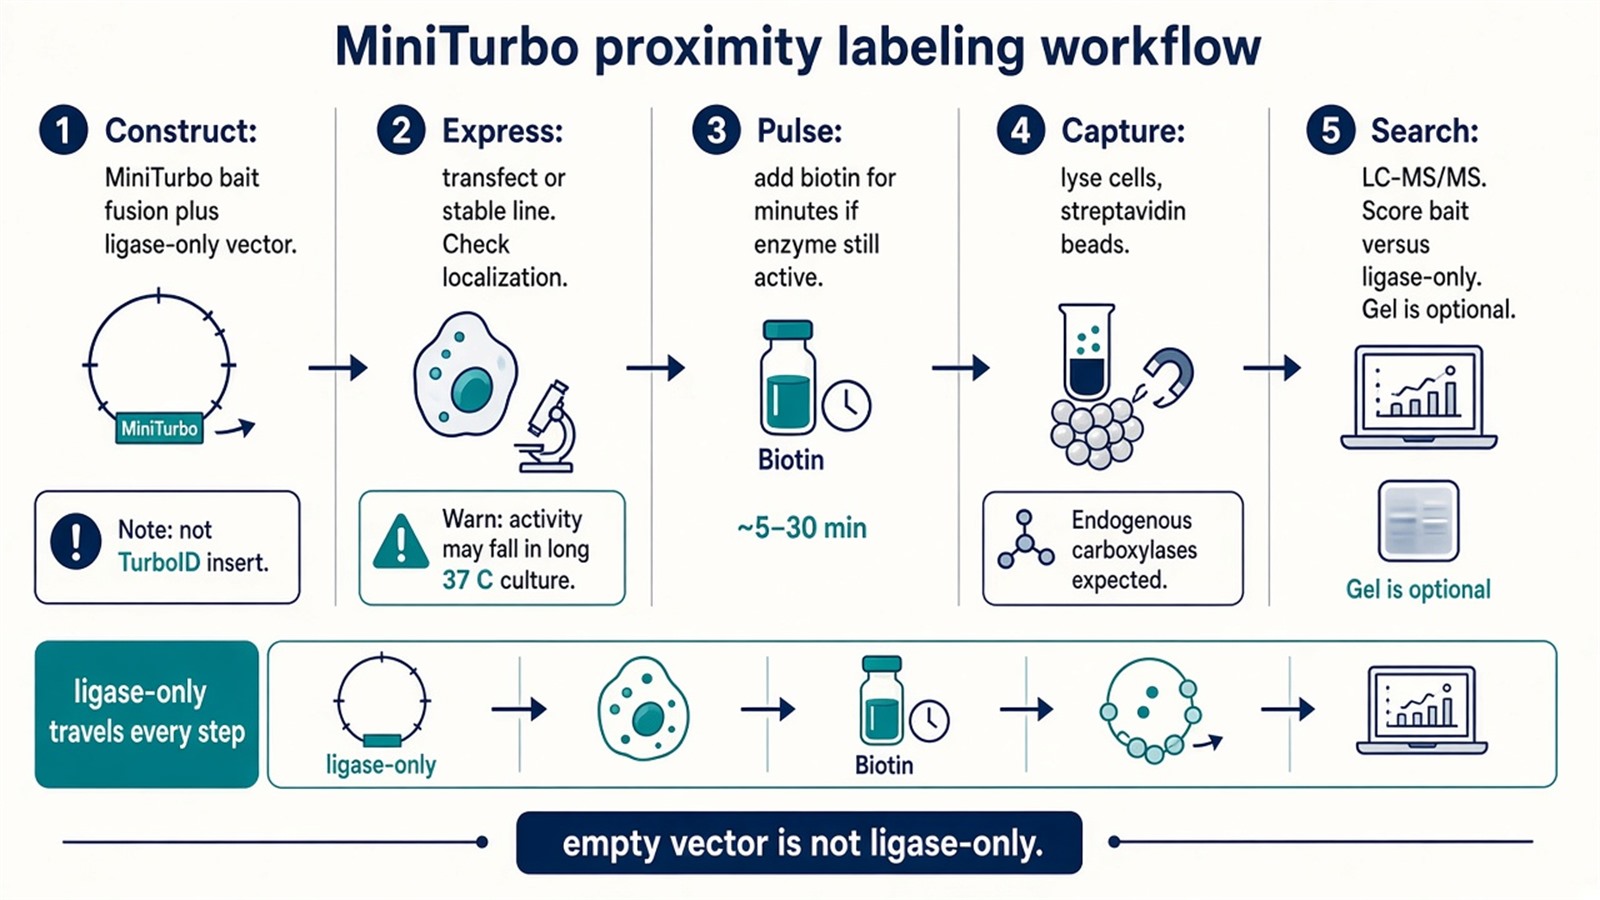
Figure 3. Vector, expression, biotin pulse, streptavidin, LC-MS/MS. Ligase-only travels through every step. A TurboID insert is a different experiment.
What the Applications Can Support
The original application list is kept only where the design matches the claim.
A bait-centered neighborhood can be listed when MiniTurbo stays on the bait and ligase-only is run. That list is not a signaling-pathway network.
A compartment or membrane-contact-site proteome can be listed when MiniTurbo is targeted to that site and a site-matched ligase-only arm is processed. Contact-site language does not become intracellular transport or signaling proof.
Protein-nucleic acid studies require a separate nucleic-acid tether or a locus-specific bait. MiniTurbo fused to a protein does not identify proteins at a genomic locus or an RNA motif.
Experimental Limits
MiniTurbo reduces a living cell to what a smaller biotin ligase fusion, a biotin pulse, streptavidin, and the search engine can report. Diagnostic, drug-discovery, and topology language sits outside ordinary research reporting unless a separately validated assay is in place.
Project Planning and Service Scope
A usable MiniTurbo plan names MiniTurbo rather than TurboID, the ligase-only arm, the biotin window, and a stability check if a long culture is planned, before the first transfection. MtoZ Biolabs scopes miniTurbo proximity labeling with Orbitrap-class LC-MS/MS. Interpretability still follows those arms, not a faster-than-BioID slogan.
Once the project may need TurboID or APEX2 as well as MiniTurbo, enzyme choice can be scoped as proximity-labeling MS. Researchers who need ligase-or-peroxidase matching can review the MtoZ Biolabs Proximity Labeling Mass Spectrometry Service for project-specific sample evaluation, feasibility assessment, and workflow planning.
Frequently Asked Questions
1. Is MiniTurbo the same enzyme as TurboID?
No. MiniTurbo is a truncated ligase from the TurboID lineage. It is smaller and often quieter before biotin. It is usually less active and less stable.
2. Does MiniTurbo label in ten minutes?
It can, if the fusion is still active. Ten minutes is also the TurboID window. Speed versus BioID is not what distinguishes MiniTurbo.
3. Is MiniTurbo more specific than BioID or TurboID?
No. Lower pre-biotin signal is not specificity. Specificity is the ligase-only comparison after the pulse.
4. Can MiniTurbo replace Co-IP for weak or transient interactions?
No. It can biotinylate a nearby protein during a short pulse. That protein is a proximity candidate, not a demonstrated binder.
5. What control should be run?
A localization-matched MiniTurbo without cargo, and where needed a no-biotin arm. Cloning TurboID, or transfecting empty vector, is not that control.
Reference
- Branon T.C., Bosch J.A., Sanchez A.D., et al. (2018). Efficient proximity labeling in living cells and organisms with TurboID. Nat. Biotechnol., 36, 880-887. https://doi.org/10.1038/nbt.4201
- Cho K.F., Branon T.C., Udeshi N.D., et al. (2020). Proximity labeling in mammalian cells with TurboID and split-TurboID. Nat. Protoc., 15, 3971-3999. https://doi.org/10.1038/s41596-020-0399-0
- May D.G., Scott K.L., Campos A.R., Roux K.J. (2020). Comparative application of BioID and TurboID for protein-proximity biotinylation. Cells, 9, 1070. https://doi.org/10.3390/cells9051070
- Roux K.J., Kim D.I., Raida M., Burke B. (2012). A promiscuous biotin ligase fusion protein identifies proximal and interacting proteins in mammalian cells. J. Cell Biol., 196, 801-810. https://doi.org/10.1083/jcb.201112098
- Gingras A.C., Abe K.T., Raught B. (2019). Getting to know the neighborhood: using proximity-dependent biotinylation to characterize protein complexes and map organelles. Curr. Opin. Chem. Biol., 48, 44-54. https://doi.org/10.1016/j.cbpa.2018.10.017
