



Interacting protein screening nominates names that were not on the prior hypothesis list. A detection technique then reads that nomination as a reporter, a band, a resonance shift, or a peptide table. The two lists on this page are not interchangeable tools that confirm interactions, discover drug targets, or provide a comprehensive view of biopharmaceutical research.
A protein library versus a bait is one screening architecture. It fits yeast two-hybrid and related display formats. It does not describe co-immunoprecipitation, crosslinking, surface plasmon resonance (SPR), or subcellular localization. Those assays test a written pair, or they return a neighborhood around one bait. They do not screen a library for proteins with specific functions.
Researchers who already have a bait and need a method match can also review the MtoZ Biolabs Protein-Protein Interaction Analysis Service for project-specific feasibility and analysis planning.
What Screening Is Allowed to Mean
The original principle has to be narrowed. Screening detects a signal that a second protein came through a written filter with the bait. It does not screen for function or potential drug targets. New interactions, protein networks, and signaling pathways are later overlays. They are not granted by running a library or an immunoprecipitate.
If the aim is unnominated names around an antibody-captured bait, the project is an IP-MS screen, not a generic detection-technique choice. For that definition, IPMS Screens for Unknown Interacting Proteins provides a complementary screen page.
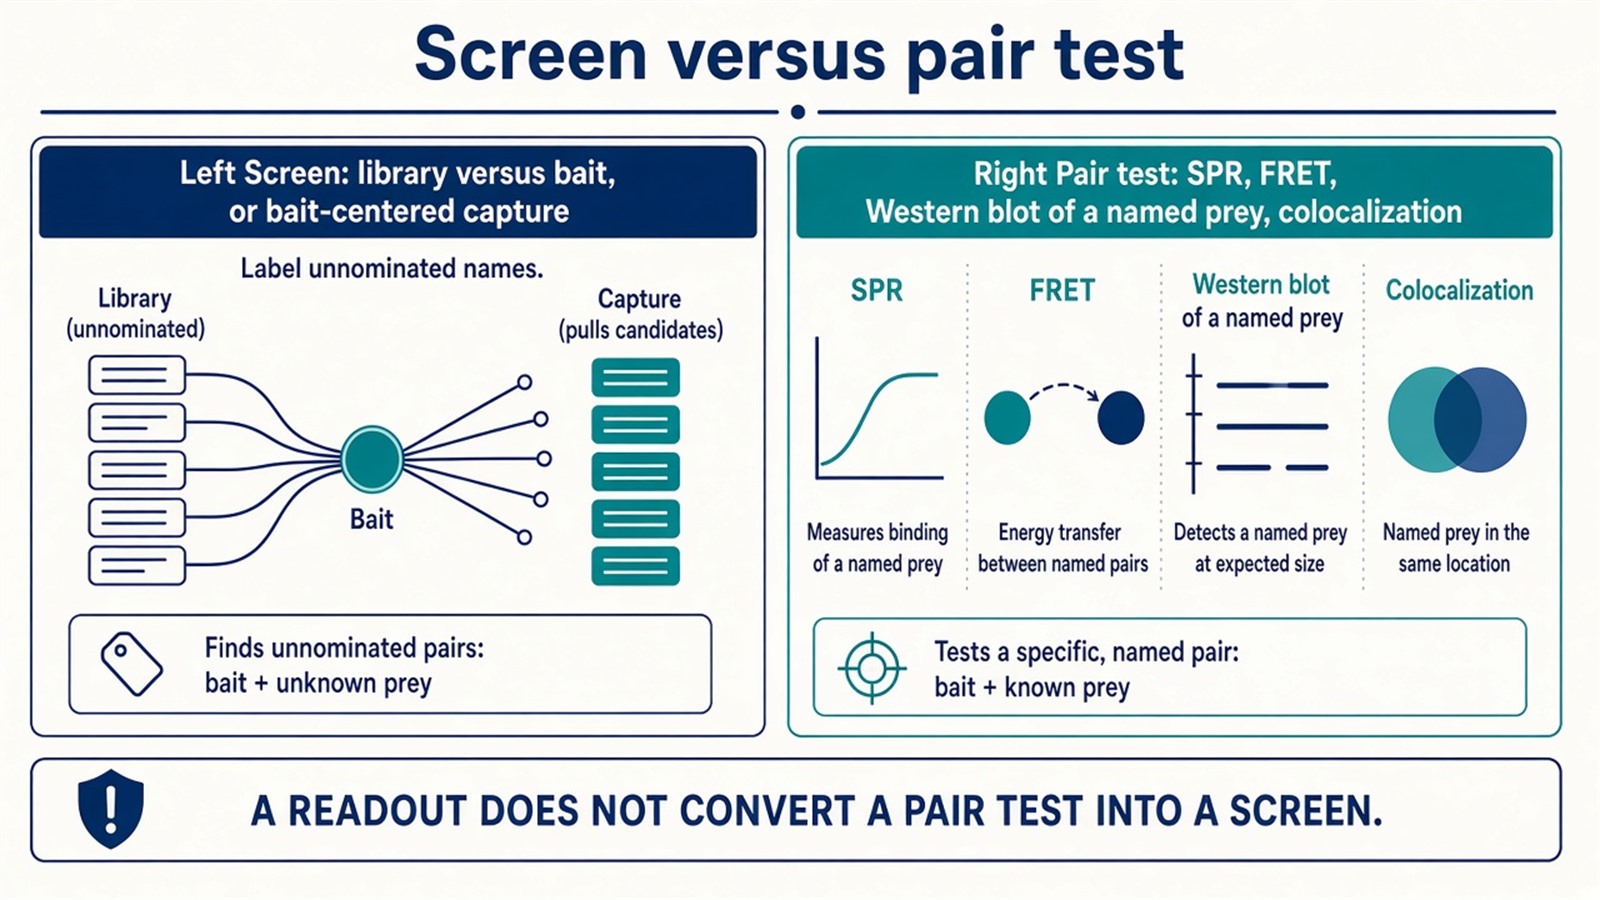
Figure 1. Library-versus-bait and bait-centered capture can nominate unknowns. SPR, FRET, Western blot of a named prey, and colocalization test a pair. They are not the same menu.
Name whether the next experiment must nominate unknowns or test a pair. A detection technique does not convert a pair test into a screen.
Common Methods, Recast
Yeast two-hybrid can screen a library. The DNA-binding domain is fused to the bait, the activation domain to library members, and a reporter fires if those fusions reconstitute in yeast. The original wording that a transcriptional activator interacts with a target protein is not the assay. Convenience, sensitivity, and high throughput are not granted. Hits are yeast-nuclear reconstitutions. They are not mammalian wash-stable partners.
Subcellular localization reports where a tagged protein sits. Colocalization with a second tag is shared address, not interaction. It cannot infer an interaction relationship, and it is not a screening method for unnominated partners.
Co-immunoprecipitation captures a bait with an antibody and pellets whatever survived the wash. With a named prey and a Western blot, it is a pair test. With LC-MS/MS against a matched isotype, it can screen unnominated names. Examining the precipitate does not identify the interaction. For that capture, How to Combine Co-IP with Mass Spectrometry for Protein Interaction Analysis? provides a complementary Co-IP-MS page.
Chemical crosslinking covalently marks residues within reach of a chosen reagent. A gel shift or a residue-pair search can follow. That is not a library screen, and it does not confirm partners by the pulse alone. SPR immobilizes one named protein and reports binding of another named protein as a resonance shift. Affinity can be fitted. SPR is not selected as a screening method for a lysate library.
Each method has a fit, not a portable advantage. Research needs still have to be written as nominate-unknowns or test-a-pair. Listing five methods and then detailing three of them, as the original page did, is how crosslinking and SPR get treated as screening tools they are not. They stay on the menu only as pair or pulse assays.
Detection Techniques, Recast
Detection techniques read a method. They do not independently confirm that protein interactions exist.
Western blot of a Co-IP pellet asks whether a nominated prey is present in that lane. It does not confirm the target protein and its interaction partners as a class, and it is not a screening technique unless many nominated preys are blotted one by one.
FRET reports whether two fluorophores came close enough for energy transfer. The proteins are already named and tagged. A change in the fluorescent signal is proximity of the dyes. It is not determination of an interaction from a screen.
Mass spectrometry, in a screening context, is usually LC-MS/MS of an enrichment. It names peptides. It does not determine interactions by analyzing spectral data of protein complexes, and it does not identify and quantify the existence of interactions. Quantification, when designed, is a contrast against a control. For the MS-route split after a screen is chosen, How to Identify Protein-Protein Interactions Using Mass Spectrometry provides a complementary method-choice page.
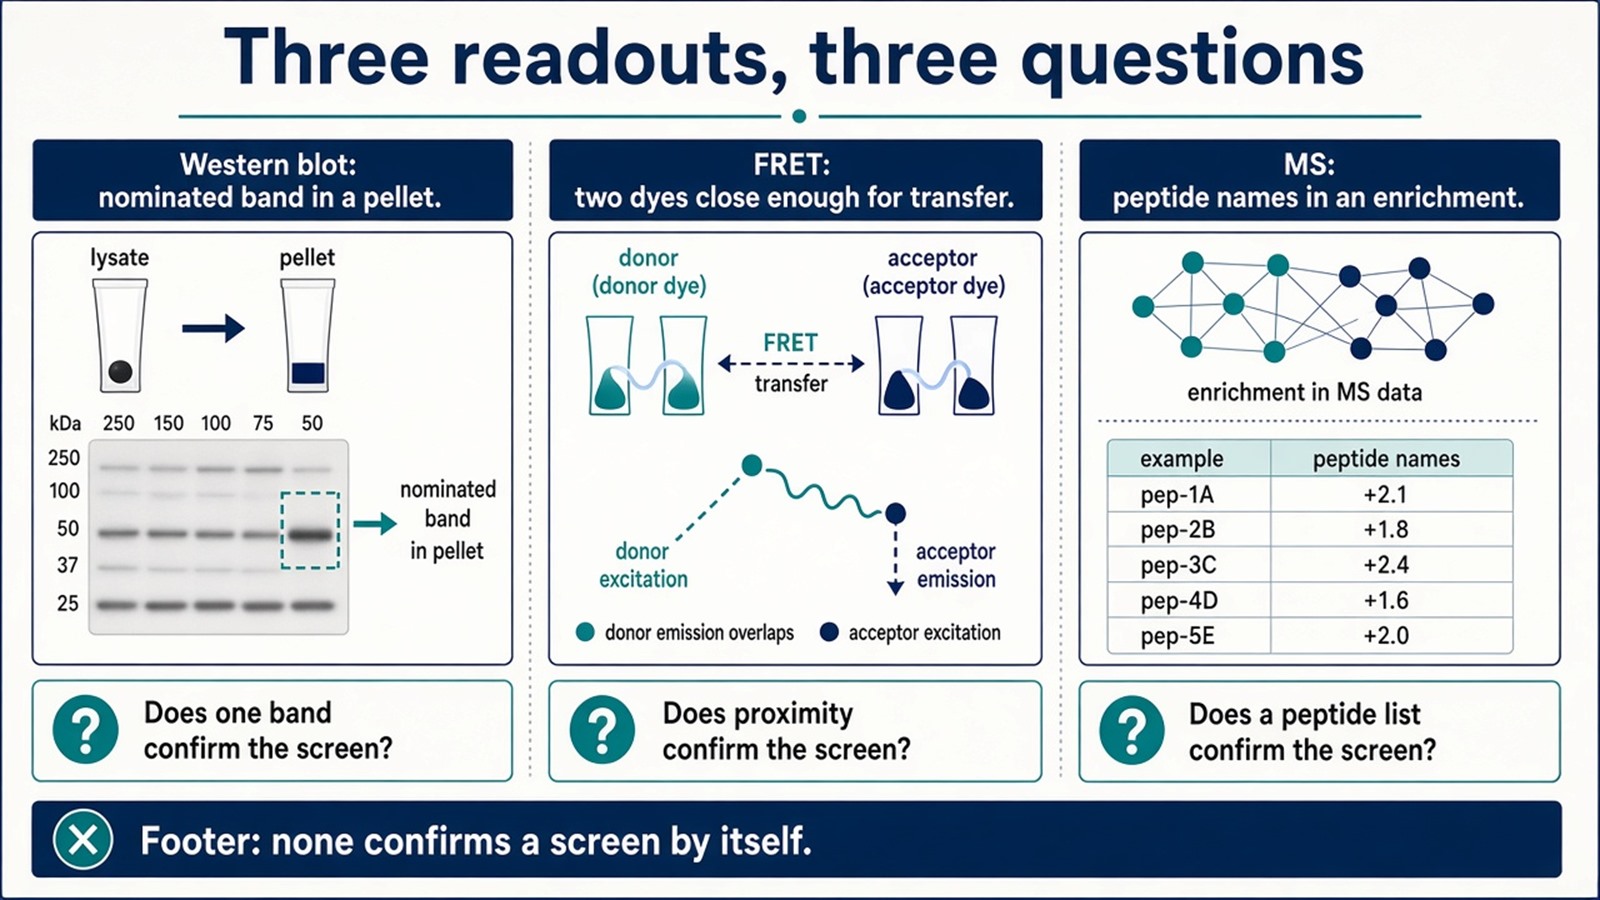
Figure 2. Western blot reads a nominated band. FRET reads dye proximity. MS names peptides in an enrichment. None of the three is a standalone confirmation of a screen.
Experimental Limits
This menu reduces a project to one screening architecture and one readout. Drug-target, network, signaling-pathway, and biopharmaceutical-foundation language sits outside ordinary research reporting unless a separately validated assay is already named. Understanding the menu does not provide a solid foundation for applications in biopharmaceuticals. A biopharmaceutical sample does not turn a pair test into a library screen, and it does not turn a peptide table into a drug target.
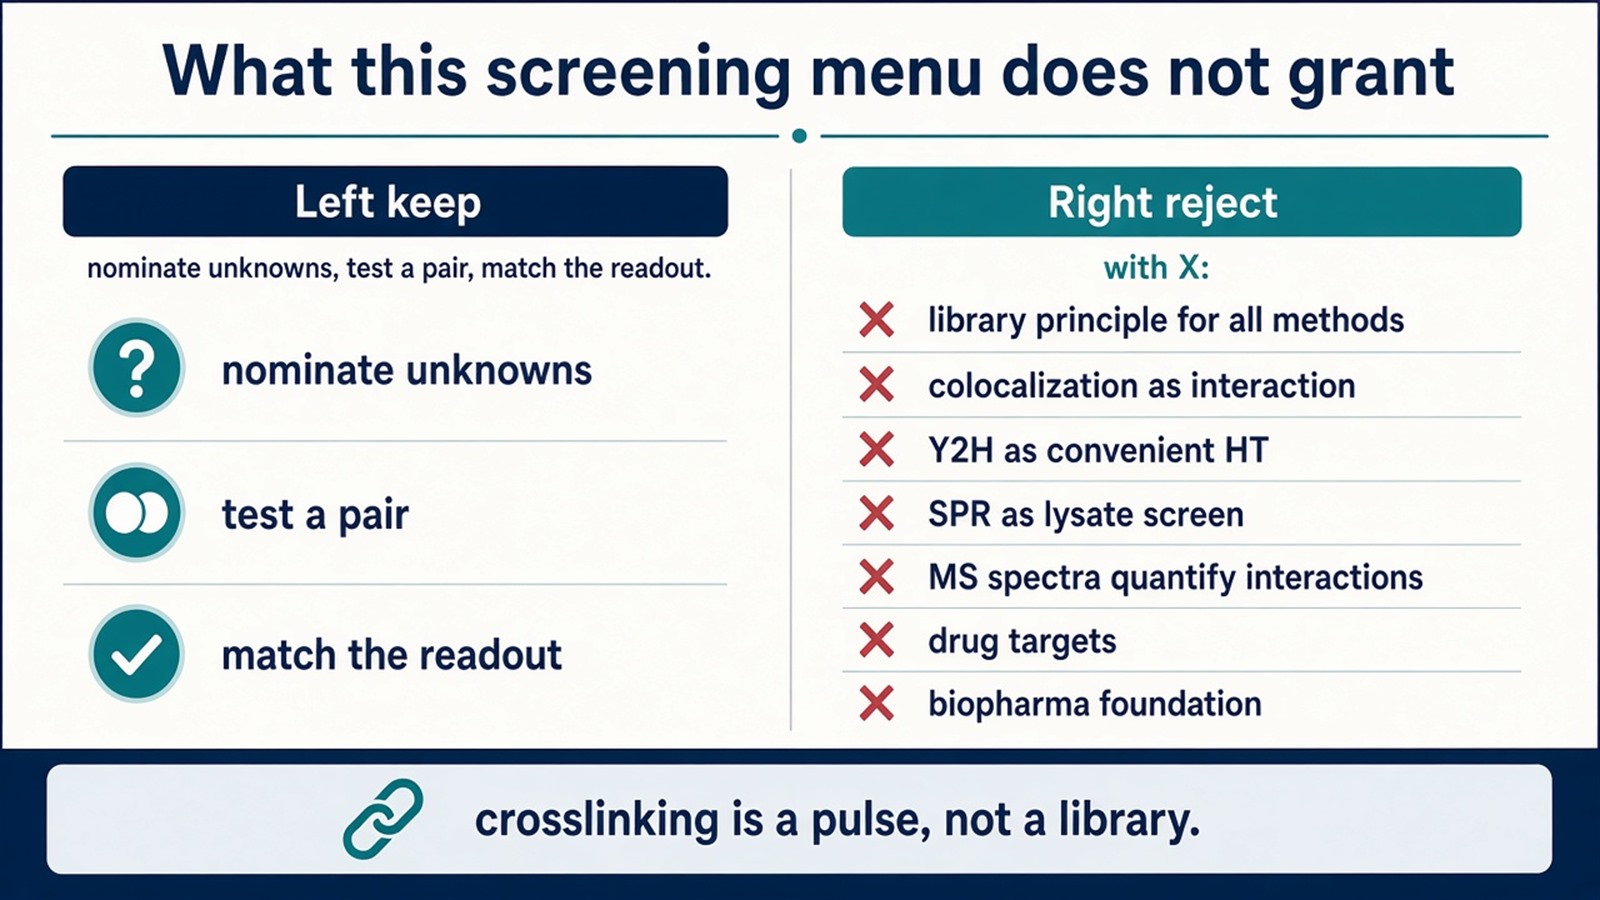
Figure 3. Keep: nominate-unknowns versus test-a-pair, then a matching readout. Not granted: localization as interaction, SPR as a library screen, MS spectra as quantified interactions, or drug-target discovery.
Project Planning and Service Scope
A usable request names whether unknowns must be nominated, the bait format, and the readout that will be allowed. If an IP-grade antibody is available and the next table should be unnominated names, the project is usually scoped as IP-MS. If only one prey is already named, a targeted Co-IP is the shorter route. MtoZ Biolabs scopes those MS files on Orbitrap-class LC-MS/MS. Interpretability still follows those arms, not a comprehensive-methods heading.
Once the next sentence is an antibody screen for unnominated names, this menu should hand off. Researchers who need that table can review the MtoZ Biolabs IP-Mass Spectrometry Service for project-specific sample evaluation, feasibility assessment, and workflow planning.
Frequently Asked Questions
1. Does protein interaction screening find drug targets?
No. It nominates names that passed a written filter. Function and target sentences need a later assay.
2. Is subcellular colocalization a screening method?
No. Shared address is not interaction, and the second protein is usually already named.
3. Can SPR or FRET screen a protein library?
Not as commonly used here. Both test a written pair.
4. Does Western blot confirm interacting partners after a screen?
It can confirm a nominated prey in a pellet. It does not confirm the screen as a class.
5. Does mass spectrometry identify and quantify interactions from complex spectra?
It names peptides in an enrichment. A ratio ranks a contrast. Existence of an interaction is a later claim.
Reference
- Fields S., Song O. (1989). A novel genetic system to detect protein-protein interactions. Nature, 340, 245-246. https://doi.org/10.1038/340245a0
- Dunham W.H., Mullin M., Gingras A.C. (2012). Affinity-purification coupled to mass spectrometry: basic principles and strategies. Proteomics, 12, 1576-1590. https://doi.org/10.1002/pmic.201100523
- Gingras A.C., Gstaiger M., Raught B., Aebersold R. (2007). Analysis of protein complexes using mass spectrometry. Nat. Rev. Mol. Cell Biol., 8, 645-654. https://doi.org/10.1038/nrm2208
- Homola J. (2008). Surface plasmon resonance sensors for detection of chemical and biological species. Chem. Rev., 108, 462-493. https://doi.org/10.1021/cr068107d
- Sekar R.B., Periasamy A. (2003). Fluorescence resonance energy transfer (FRET) microscopy imaging of live cell protein localizations. J. Cell Biol., 160, 629-633. https://doi.org/10.1083/jcb.200210140
